By Amara Williams
Few ideas in nutrition science have had a longer public life than the notion that everyone carries around a personal, biologically fixed body weight. The phrase “set point” shows up in gym conversations, diet books, and clinical waiting rooms alike, usually deployed as an explanation for why weight loss stalls or why lost pounds seem to find their way back. The concept is compelling because it matches lived experience: most people who lose a meaningful amount of weight regain some or all of it within a few years. But the scientific story behind that experience is more layered than the popular version suggests, and researchers have spent decades arguing over how rigid, how adjustable, and how biologically “real” a weight set point actually is.
This review walks through what the evidence actually supports, where the classic set point model runs into trouble, and how an alternative called the settling point model — along with a middle-ground “dual intervention point” framework — has reshaped the conversation among obesity researchers. The goal is not to declare a winner but to describe the current state of a genuinely unsettled scientific debate, one where the honest answer to “is there a set point” is closer to “partly, and it depends what you mean by the term” than a clean yes or no.
Understanding why this matters goes beyond academic curiosity. People trying to lose fat and keep it off often interpret a stall or a rebound as personal failure, when the underlying biology may be doing exactly what decades of research would predict. Knowing which parts of that biology are fixed, which parts respond to sustained behavior change, and which parts are shaped by food environment and daily habits changes how realistic, and how forgiving, a long-term approach to weight management can be.
The Biological Basis: Leptin and Hypothalamic Regulation
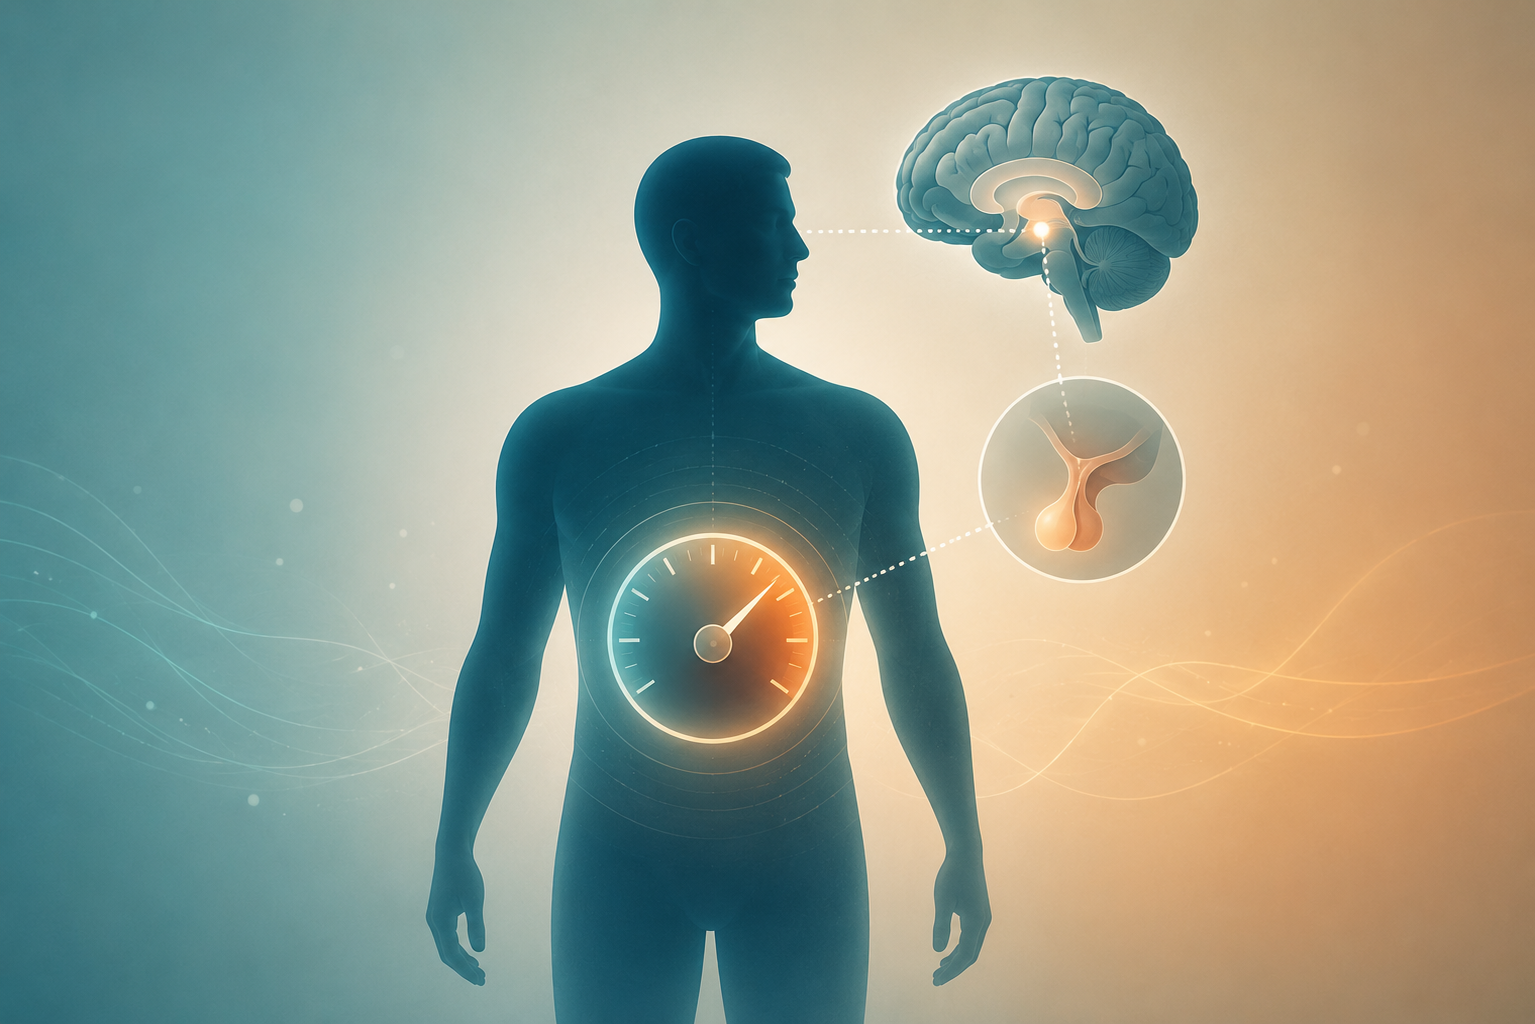
The modern version of set point theory rests heavily on the discovery of leptin, a hormone secreted by fat cells that circulates in the bloodstream roughly in proportion to total body fat. Leptin was identified in the mid-1990s and quickly became the centerpiece of body weight research because it gave scientists a measurable biological signal connecting fat stores to brain activity.
How Leptin Signals Energy Status
Leptin travels to the hypothalamus, a small structure at the base of the brain that coordinates hunger, satiety, and energy expenditure. In the lateral hypothalamus, rising leptin levels inhibit hunger signals partly by counteracting neuropeptide Y (NPY), a potent appetite-stimulating peptide produced in the arcuate nucleus. NPY acts through Y1 and Y5 receptors to increase food intake and fat storage, while Y2 and Y4 receptor activity tends to suppress appetite. In the medial hypothalamus, leptin promotes synthesis of alpha-MSH, a compound that further suppresses hunger. When leptin signaling to these circuits works as intended, energy intake and expenditure track fat mass fairly closely over time.
The Hypothalamic Circuitry and Leptin Resistance
The relationship breaks down in a well-documented way. In obesity, circulating leptin is typically high rather than low, because more fat tissue produces more leptin, yet the brain often fails to register the signal appropriately. This state, commonly called leptin resistance, resembles insulin resistance in type 2 diabetes: the hormone is present in abundance, but downstream signaling — largely through the JAK-STAT pathway — does not translate into reduced hunger or increased energy expenditure. Researchers have also noted that leptin’s role appears asymmetric: levels fall more sharply during calorie restriction than they rise during overfeeding, which has led some scientists to describe leptin less as a fullness signal and more as a starvation alarm that becomes far more active when fat stores drop.
Evidence Summary
- Leptin falls faster with weight loss than it rises with weight gain, consistent with a starvation-defense function.
- Genetic leptin deficiency reliably causes severe obesity in humans and animals, but this defect explains only a small share of obesity cases.
- Leptin resistance in common obesity appears to involve impaired JAK-STAT signaling rather than a simple lack of leptin.
- The 1950 Minnesota Starvation Experiment showed subjects regaining weight well beyond their pre-starvation baseline after refeeding, a pattern often cited as support for defended weight ranges.
- Speakman and colleagues’ 2011 review proposed that most body weight regulation reflects a “settling point” driven by passive feedback, not a fixed biological target.
What Set Point Theory Explains Well
Set point thinking earns its continued relevance because certain observations line up with it consistently across studies and clinical populations.
The Tendency to Regain Lost Weight
The most frequently cited support for a defended weight comes from what happens after substantial weight loss. Metabolic rate tends to drop by more than body composition changes alone would predict, a phenomenon researchers call adaptive thermogenesis. Skeletal muscle in particular shows notable metabolic plasticity during dieting, persistently reducing its energy expenditure in ways that outlast the diet itself, a mechanism described by Summermatter and Handschin in 2012. Appetite-regulating hormones shift in a direction that favors regain: hunger signals strengthen while satiety signals weaken, and this hormonal profile can persist long after active dieting ends. The classic illustration remains the Minnesota Starvation Experiment conducted by Ancel Keys and colleagues in the late 1940s, in which severely calorie-restricted men regained weight after refeeding until they reached roughly 145 percent of their original fat mass before gradually settling back down, a rebound pattern that is hard to explain without invoking some form of active biological compensation.
Defended Ranges and Compensatory Responses
Beyond simple regain, researchers have documented compensatory responses in both directions. Overfeeding studies show that some individuals increase spontaneous physical activity and resting energy expenditure when force-fed excess calories, resisting weight gain to a degree. Underfeeding produces the opposite: reduced activity, reduced resting expenditure, and heightened hunger. Rachel B. Harris’s influential 1990 review in the FASEB Journal framed this two-directional resistance as evidence of active regulation around a defended range rather than passive drift. Experiments knocking down leptin receptors specifically in the lateral hypothalamus of rats produced overeating and weight gain, reinforcing the idea that this circuit actively defends against weight loss below some threshold, even if it defends less forcefully against weight gain above it.
Genetic Contributions and Twin Studies
Some of the strongest support for a heritable, individually variable regulated weight comes from twin research rather than hormone assays. Albert Stunkard and colleagues’ 1990 study of twins reared apart, published in the New England Journal of Medicine, found body mass index correlations among identical twins raised in separate households that approached those of identical twins raised together, with heritability estimates in the range of 60 to 70 percent. That finding is hard to explain through shared household food environment alone, since the twins in question did not share a household. A related overfeeding study by Claude Bouchard and colleagues, also published in the New England Journal of Medicine in 1990, deliberately overfed pairs of identical twins by a fixed number of calories over several months. Weight gain varied widely between twin pairs, from roughly four pounds to nearly thirty, but was strikingly similar within each pair, and the twins even tended to store the extra fat in similar body regions. That pattern suggests a genetically influenced response to a calorie surplus, though it says less about whether that response reflects a fixed set point or simply a genetically influenced settling point, since both models can accommodate the idea that genes shape how strongly the body resists or accommodates a calorie surplus.
Where the Theory Is Contested
For every observation that appears to support a fixed, actively defended weight, there is a competing explanation, and several aspects of the classic model have not held up well under scrutiny.
The Settling Point Alternative
The most substantial challenge came from a 2011 paper by John Speakman and colleagues in Disease Models and Mechanisms, which argued that much of what looks like active defense of a set weight can be explained by passive settling dynamics instead. Larger bodies burn more energy at rest, require more energy for movement, and interact with a fixed food environment in ways that naturally push weight toward an equilibrium, without any biological target being consulted. Under this settling point model, body weight rises or falls until intake and expenditure happen to balance again, and where that balance point lands depends heavily on the food environment, activity level, and habitual behavior rather than a preset internal value. This reframing matters because it shifts the emphasis from an unchangeable internal thermostat to a movable equilibrium shaped substantially by circumstance.
Behavioral and Environmental Influences
Population-level weight trends are difficult to reconcile with a purely biological set point. Average body weight has shifted upward across many countries over a few decades, a period far too short for large genetic change, pointing instead toward environmental drivers such as food availability, portion sizes, food composition, and reduced physical activity demands in daily life. Socioeconomic differences in obesity prevalence within the same country and genetically similar population also argue against a rigid internal set point as the dominant explanation, since a fixed biological target should not vary so strongly with income, occupation, or neighborhood food access. Sleep restriction and chronic stress add another layer: raised glucocorticoid levels stimulate neuropeptide Y synthesis directly, and studies have found higher levels of free NPY in obese women compared with leaner women, suggesting environmental and psychological stressors can push the regulatory system toward fat storage independent of any single defended value.
Non-Exercise Activity and the Food Environment
Research led by James Levine at the Mayo Clinic on non-exercise activity thermogenesis, commonly shortened to NEAT, adds another environmental thread to this debate. NEAT covers the energy spent on fidgeting, posture maintenance, walking during daily chores, and other movement that falls outside structured exercise, and it varies enormously between individuals, by several hundred calories a day in some comparisons. Levine’s overfeeding studies found that people who spontaneously increased NEAT in response to extra calories gained less fat than those whose NEAT stayed flat, pointing to a partly automatic, partly behavioral buffer against weight gain that has nothing to do with a fixed internal target. The rise of highly palatable, energy-dense, minimally satiating food products across the food supply works in the opposite direction, encouraging higher passive calorie intake without a matching rise in fullness signals. Taken together, NEAT variability and food environment changes give the settling point model a mechanistic story for why average population weight can shift over just a few decades, a timescale far too short for meaningful genetic change but entirely plausible for a system that settles wherever intake and expenditure happen to balance.
A Middle Ground: The Dual Intervention Point Model
Some researchers have proposed a compromise between rigid set points and fully passive settling. The dual intervention point model suggests the body defends a range bounded by an upper and lower threshold rather than a single number. Within that range, weight can drift with behavior and environment largely unchecked. Once weight approaches either boundary, active compensatory mechanisms — the hormonal and metabolic responses described above — become more forceful. This model helps explain why short-term weight fluctuations of a few pounds provoke little biological pushback while larger, sustained changes trigger stronger resistance, particularly on the downward side.
| Feature | Set Point Model | Settling Point Model |
|---|---|---|
| Core claim | Body actively defends a specific target weight | Weight equilibrates passively based on intake and expenditure feedback |
| Role of environment | Secondary to internal biology | Primary driver of where weight settles |
| Explains weight regain | Yes, via active hormonal defense | Yes, via mass-dependent metabolic changes |
| Explains rising population weight | Poorly, since biology changes slowly | Well, since equilibrium shifts with food environment |
| Practical implication | Weight loss fights biology | Weight loss requires changing the equilibrium conditions |
| Key proponent(s) | Harris (1990); early leptin researchers | Speakman et al. (2011) |
Practical Implications for Long-Term Fat Loss
Whichever model turns out to describe the underlying biology more accurately, the practical picture for someone trying to lose fat and keep it off is fairly consistent across both frameworks. Sustained weight loss tends to trigger hormonal and metabolic changes that increase hunger and reduce resting energy expenditure, regardless of whether those changes are labeled active defense or passive adjustment. That means the period after weight loss, not just the loss itself, deserves deliberate planning: preserving muscle mass through resistance training helps offset some of the drop in resting expenditure, since muscle tissue is metabolically active and responsive to training stimulus. Gradual, smaller calorie deficits sustained over longer periods appear to provoke less severe hormonal pushback than steep, rapid restriction, and gradual reintroduction of calories after a diet phase gives the hunger and satiety systems more room to recalibrate.
Sleep and stress management matter more than they are often given credit for for reasons directly tied to the neuropeptide Y pathway described earlier. Chronic short sleep and raised stress hormone levels both push the appetite system toward greater food-seeking behavior, working against whatever ground has been gained through diet and exercise. Building an eating and activity pattern that can be maintained indefinitely, rather than one designed only to reach a short-term number, aligns with the settling point view that where weight lands depends heavily on the conditions maintained over time. Under the dual intervention point framework, this also means that modest weight loss goals sitting within a person’s existing defended range may be easier to sustain than large losses that push near a lower boundary the body actively resists.
Protein intake deserves specific mention because it interacts with several of the mechanisms already described. Diets that keep protein relatively high during a calorie deficit tend to blunt lean mass loss and support satiety more effectively than lower-protein diets at the same calorie level, which can partly offset the drop in resting expenditure and the rise in hunger signaling that typically follow weight loss. Regular self-monitoring, whether through periodic weigh-ins or simple food tracking, gives an early warning system for the small, steady regain that often precedes larger rebounds, allowing adjustments before the defended range fully reasserts itself. None of these tools override the underlying biology, but they work with it rather than against it, which the twin-study and settling point evidence both suggest matters more than any single tactic.
Expectation-setting also matters clinically. A person who understands that a plateau after six months of steady loss is a predictable, well-documented biological response, not a sign that effort has stopped working, is more likely to adjust calories or activity modestly rather than abandoning the approach altogether. Clinicians and coaches who frame plateaus this way tend to see better long-term adherence than those who treat every stall as a behavioral lapse.
Conclusion: A Balanced Current Understanding
The evidence supports a version of body weight regulation that sits between the two extremes of a rigid, unchangeable set point and a purely passive drift with no biological resistance at all. Leptin, the hypothalamus, and related appetite hormones clearly create real physiological pressure that favors weight regain after loss, particularly through mechanisms like reduced resting metabolism and heightened hunger signaling. At the same time, the magnitude of that pressure, and where the body ultimately settles, depends substantially on food environment, activity patterns, sleep, stress, and behavior over months and years, not on a single fixed number written into a person’s biology at birth. Framing body weight as a defended range shaped by both physiology and circumstance, rather than as an immovable set point, matches the available data more closely and offers a more actionable picture for anyone working toward long-term fat loss.
Frequently Asked Questions
Is set point theory scientifically proven?
Not in the strict sense. The core biological mechanisms — leptin signaling, hypothalamic appetite circuits, adaptive drops in resting metabolism — are well documented in both animal and human research. What remains unproven and actively debated is whether these mechanisms defend a truly fixed target weight or instead produce a flexible equilibrium that shifts with environment and behavior, as the settling point model proposes.
Can a person’s set point change over time?
Under the dual intervention point model, the defended range itself can shift gradually with sustained changes in body composition, activity, and diet quality maintained over long periods. Rapid crash dieting does not appear to reset this range quickly, which is part of why quick, aggressive weight loss so often reverses.
Does leptin resistance mean more leptin would help with weight loss?
Generally no. Most people with obesity already have high circulating leptin, so the issue is impaired signaling rather than insufficient hormone. Supplemental leptin has shown limited benefit in typical obesity, though it can be effective in the rare cases of genetic leptin deficiency.
Why do some people regain weight faster than others after dieting?
Individual variation in hormonal response, muscle mass retention, sleep quality, stress exposure, and food environment all influence how strongly the appetite and metabolism-related compensations kick in after weight loss, which is one reason outcomes differ so much between individuals following similar diets.
Does exercise change the set point or settling point?
Exercise, particularly resistance training, helps preserve lean muscle mass during weight loss, which supports resting energy expenditure and may make a lower body weight easier to maintain. It does not appear to eliminate the hunger and metabolic adaptations that follow substantial fat loss, but it can offset part of their impact.
Is the settling point model widely accepted among obesity researchers?
It is one of several competing frameworks taken seriously in the field, alongside the dual intervention point model and more traditional set point language. Current scientific statements, including the Endocrine Society’s 2017 position on obesity pathogenesis, tend to describe body weight regulation as a system shaped by both biology and environment rather than endorsing any single model exclusively.
References
- Harris, R. B. (1990). Role of set-point theory in regulation of body weight. FASEB Journal, 4(15), 3310-3318.
- Keys, A., Brozek, J., Henschel, A., Mickelsen, O., & Taylor, H. L. (1950). The Biology of Human Starvation. University of Minnesota Press.
- Speakman, J. R., Levitsky, D. A., Allison, D. B., et al. (2011). Set points, settling points and some alternative models: theoretical options to understand how genes and environments combine to regulate body adiposity. Disease Models & Mechanisms, 4(6), 733-745.
- Summermatter, S., & Handschin, C. (2012). PGC-1alpha and exercise in the control of body weight. International Journal of Obesity, 36(11), 1428-1435.
- Schwartz, M. W., Seeley, R. J., Zeltser, L. M., et al. (2017). Obesity Pathogenesis: An Endocrine Society Scientific Statement. Endocrine Reviews, 38(4), 267-296.
- Harvard Health Publishing. Why people become overweight.